1. The model in five lines
The Sensible Universe Model (SUM) says that reality has two parts, not one. There is the measurable world of space and time — M₄. And there is a
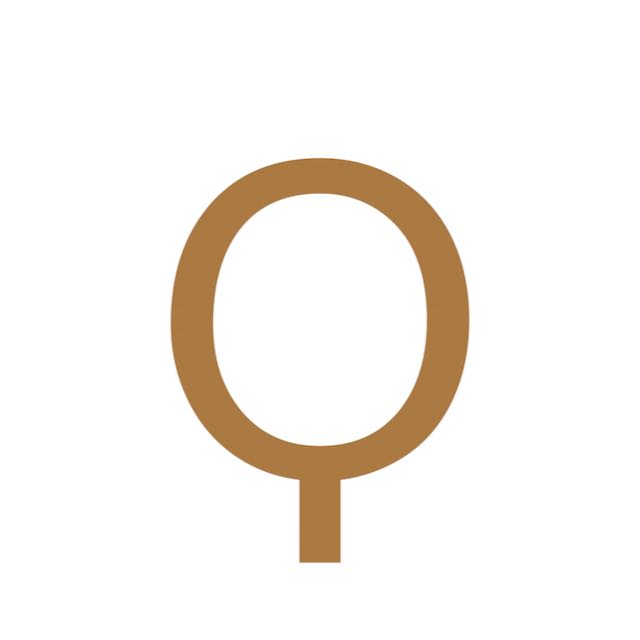
second dimension alongside it — Ϙ, the qualitative dimension: the arena in which felt experience occurs. The two always come together:
M₅ = M₄ × Ϙ
Inside Ϙ there is a field, the Primaton field (Π_Ϙ). Its quantum is the
Qualiton (q) — one unit of felt quality. And the field has a ground state
that is not zero. That non-zero ground is Λω — Amor, Love. Not love as
an emotion: love as the ground of reality. It shows itself in three aspects:
Logos (love as intelligible), Aletheia (love as self-disclosing), and
Iustitia (love as right proportion).
Experience enters at the boundary of Ϙ (∂Ϙ): five gates, and only five —
sight, sound, smell, taste, touch. What crosses a gate from the physical world is the Sensibiliton (σ). What arrives, felt, is a Qualiton — one of five
kinds: chromaton (sight), akouoton (sound), osmeton (smell),
gefseton (taste), kinestiton (touch). A carrier called the Lomegon
(λ) brings the ground signal, Λω, into each gate.
And there is a witness — Position Zero (P₀): undetermined, invariant, the
point where things are resolved. It rests in D∞, the unbounded.
That is the whole model in outline. This page asks one question: what does any of this have to do with biology?
2. The boundary of the living body
Here is the first answer, and it is simple. The five gates are not
abstractions. They are built by living bodies. Every eye, ear, nose, tongue
and skin is a biological structure whose whole job is ∂Ϙ — the boundary of
the qualitative dimension.
The eye does not see light as physics describes it. It receives photons and
presents them, at the gate of sight, as colour. The ear receives pressure
waves and presents them as sound. The skin receives contact and presents it as touch. On the physical side of each gate there is chemistry and
electricity. On the other side there is what it is like. Biology is the
machinery of the crossing.
SUM adds one claim: nothing crosses unless it fits. The formal name is
Fit (κατάλληλος, katallilos written ⋈) — recognition, the condition in which something is received completely as what it is. A key that does not fit the lock does not open the door, and a signal that does not fit the receptor does not arrive. Fit is a relation, not a quantity.
Biology already has this idea. It just calls it by other names.
3. Molecular recognition: Fit under the microscope
In 1894, Emil Fischer described enzymes and their targets with the image of a lock and key: only the right key enters the right lock. In 1958, Daniel
Koshland refined the image to induced fit: the lock bends a little as the
key goes in, so that two things come to fit each other. These two ideas —
molecular recognition, as biology calls the whole family of them — are the
small-scale mechanics of what SUM calls Fit.
Look at the most important recognition event in the body: the pairing of the letters of the genetic code. In RNA there are four letters — A, U, C, G. A pairs with U, held by two hydrogen bonds. G pairs with C, held by three.
Nothing else pairs. A single hydrogen atom, placed or absent at the right
spot, is the difference between a match and a mismatch. Every time a cell
reads its genes, it is performing, trillions of times over, a vast act of
molecular recognition — lock and key at the scale of single atoms.
Three letters at a time make a codon, and each codon names one of twenty
amino acids, the building blocks of proteins. Three letters is the smallest
number that works: one letter gives only 4 possibilities, two give 16, three
give 64 — enough for all twenty, with room to spare.
SUM’s reading: recognition is not a metaphor borrowed for consciousness. It is the same thing at every scale. Where biology sees a lock and key, SUM sees Fit — x ⋈ y, two things meeting on what they share. The hydrogen bond that holds A to U is the smallest worked example of what happens at every gate of perception: what does not fit does not cross; what fits, arrives.
This is the model’s entry point into biology, and it stays deliberately
modest. Chemistry does everything chemistry is said to do. SUM does not
dispute a single result of molecular biology. It asks a second question
alongside the chemical one: why is recognition so fundamental, so universal, so carefully preserved — everywhere, at every scale?
4. Evolution: selection is selection for Fit
Mainstream biology says that variation is random and the environment selects. SUM does not dispute the mechanism. It reads it differently.
What survives, survives because it fits. Organisms fit their environments — that is ordinary Darwinism. But beneath the organism, chemistry has its own fits: bases that pair, codons that code, proteins that fold into shapes that recognise their partners. Evolution is not free to wander anywhere. It can only ever build with what fits.
This is why the same solutions keep appearing independently. The camera eye arose separately in vertebrates and in octopuses. Streamlined bodies arose separately in fish, dolphins and ichthyosaurs. If evolution were genuinely random, deep repetition of this kind would be astonishing. If evolution is a search among what fits — among locks that already have keys — repetition is what you expect: different roads arriving at the same door.
So SUM’s claim about evolution is not that it is guided. It is that it is
channelled. The space of workable biology is far narrower than a purely
neutral chemistry would suggest, and evolution keeps finding the same narrow places. Evolution did not invent molecular recognition. It discovered it, again and again, because recognition is where chemistry works.
5. Kardioton: the heart’s own reading
There is a reading that does not come through any of the five gates. The
Index calls it Kardioton — the felt registration of one’s own heartbeat —
and has moved the term here, to biology, because there is a real biological
relation between cardiac state and emotion, and the term belongs with it.
Everyone knows the phenomenon. Fear is not only an idea that something is dangerous; it is the heart going. Calm is not only an absence of alarm; it is the heart slowing. The relation between heart and feeling is two-way and is now actively studied — but you did not need the studies to know it exists. You have a heart.
In SUM’s terms, Kardioton sits beside the gates rather than inside them. The five gates register what crosses from the world; the heart’s reading registers the state of the field that receives. It is the body’s simplest reminder that not everything felt arrives from outside.
6. The touch gate and care
Of the five Qualitons, the kinestiton — touch — has a special case that
deserves its own line. In human skin there are nerve fibres, the C-tactile
afferents, that respond not to pressure or pain but to gentle, warm, slow
touch — exactly the touch of being stroked or held. They are wired toward the emotional centres of the brain, not the analytical ones. Their signal is
carried slowly, and it is felt as comfort, as being with.
Every mammal that tends its young uses this channel. It is the clearest
biological case of a Qualiton that arrives already carrying weight: the touch is not just contact, it is care. The Index lists these fibres among the
model’s borrowed biology, and rightly — they are established science. What SUM adds is only the placement: of all the things that cross the gates of a living body, gentle touch is the one nature most obviously built for receiving love with.
7. Memory beyond the gene
A third borrowed term from the Index: epigenetic transmission.
DNA is the archive, but it is not the only form of inheritance. Cells mark
their genes with chemical tags — turning them up or down without changing the sequence — and some of these marks pass to daughter cells, and in some cases across generations. Experience leaves chemical traces that outlast the experience.
SUM attends to this for one reason. The model’s central claim is that there is a non-zero ground to experience — Λω — and that events at the boundary carry weight. Gravitas accrues to the one who chooses; GRAVIS is the weight of what crossed. Epigenetics is the closest mainstream biology comes to saying that what happens to a living thing leaves a mark on what it passes on. The model does not claim that GRAVIS is an epigenetic mark. It notes the structural echo: weight, carried forward, in matter.
8. Awareness from cell to witness
The Index defines Percatar as awareness — active registration with a
minimum of interiority — and says it is continuous, from the cell to the
witness of the witness.
Biology knows the cell’s end of that continuum well. A cell surveys its
surroundings constantly. It recognises molecules, distinguishes self from
other, repairs damage, and responds. The immune system performs recognition across the whole body with a precision that still outclasses engineering. None of this proves the cell has experience — SUM does not claim it does. The claim is narrower and stranger: that registration is one thing, appearing at many depths, and that the witness at Position Zero is not a new kind of entity added on top of biology, but the same registration arrived at full clarity.
You do not need to accept that to keep reading. It is the model’s wager, and it is marked as such.
9. Felt weight: GRAVIS and the readings
Finally, three terms for what the field registers in itself — not crossings,
but readings of the field’s own state. Biology meets all three.
Synaisthiton — coherence: the strong registration of inner reality, as in
profound contemplation. What follows it is Tetelestai: it is finished,
weight carried to completion.
Entheusiton — surplus: felt weight exceeding what the occasion accounts
for, read as pleasure or as pain — and it has a limit beyond which the organ is destroyed. Here biology and the model say the same sentence. Pain is the body’s reading of excess; a pain that never ends destroys the tissue that reports it; chronic stress damages the very organs that carry the alarm. The Entheusiton is not an ornament on the model. It is the body’s homeostasis, named from the other side.
Agapiton — the shared ground: the reading that the ground is common
between two conscious fields. Biology’s version is the whole of social
biology — the recognition of another, the fits between minds. The model claims only that this, too, is a reading of something real: that between two fields, the ground is one.
And GRAVIS — the ontological weight of an experience — has its direct
measure in felt time: how fast the present advances. Qualitative time,
τ_Ϙ, runs against the clock, and the ratio W(τ) between them measures the weight. Biology knows this from inside: an hour of pain and an hour of joy are not the same length. The clock disagrees. The model sides with you.
10. The curves of violence
Evil cannot be measured. Violence can — because violence is behavior, and
behavior leaves records. This section gathers what the records show, in two
parts, because the data itself falls into two parts.
Part one: the mechanics — the vehicle
The first part of the data concerns the vehicle of violence: how it moves,
regardless of what it is carrying. The curves here are among the most regular in social science.
Violence rises and falls with temperature — up to a point, then no further.
It rises past a threshold with alcohol, not proportionally. It peaks in the
late teens and declines with age. Its risk is highest immediately after a
release or a war, and decays with every clean year — the same recurrence
curve in the prison and in the peace table. And people leave violence, most
reliably, when they acquire fit: steady work, a bond, a self they can
narrate.
The vehicle has no opinions. The same mechanics carry a bar brawl, a riot and a war. In the model’s language, this part of the data is the physics of
deformation: load applied to a field, curvature accumulating (GRAVIS), the surplus read as pain when it crosses the limit (Entheusiton). The curves are lawful because the vehicle is lawful.
Part two: the content — what is carried
The second part of the data concerns what the violence is about — and here
the curves go quiet. Mechanics can tell you when a crowd will turn violent.
It cannot tell you why this crowd names its wound as sacred.
Religious and political violence are the hard cases, and the data explains
why. In ordinary conflict, the parties disagree over positions. In conflict
where the content claims ultimacy — a creed, a flag, a people identified with the highest good itself — the opponent is no longer mistaken. The opponent is against the ground. Misfit (ἀκαταλληλότης) becomes total, and total misfit does not bargain. The research on sacred values says exactly this: such conflicts resist material compromise, and they soften under symbolic recognition — a gesture, not a payment. SUM reads this as the signature of content that has identified a position with Λω itself. The position then borrows the ground’s ultimacy, and the conflict recurs — the recurrence curve again — because a phase difference over the ground can be suspended but never settled by mechanics alone.
Resolution needs both
This is the practical consequence, and it is strict. Mechanics answer to
mechanics: cooling, contact, repeated interaction, structures that restore
fit — work, law, trade. Content answers only to content: re-reading,
recognition, the recovery of a ground both sides can register as shared.
Each failure mode has its own fingerprint. A ceasefire that recurs is
mechanics without content — the phase difference was shelved, not resolved. A riot is content without mechanics — a crowd whose vehicle is already moving cannot be argued with, only cooled. Lasting peace is both at once: curvature relaxed over years (the GRAVIS decay), and shared ground actually recovered (the Agapiton reading — the field registering that the ground between two conscious fields is one).
The Index’s Conflict Resolution Conjecture names this from the model’s side: conflict is a phase difference between qualitative fields, resolution is the convergence of phases, and the hermit retreat is the proposed mechanism. This page borrows the conjecture only at the scale where it meets the data: the curves say that convergence is slow and decays under neglect; the conjecture says why it is possible at all.
11. What this page claims — and what it does not
The Index distinguishes two kinds of term, and this page keeps the
distinction.
Borrowed — lock and key (Fischer, 1894), induced fit (Koshland, 1958),
molecular recognition, C-tactile afferents, epigenetic transmission: these
belong to biology and mean what biology means by them. Nothing here disputes or amends them.
The model’s own — M₅, Ϙ, the Primaton field, Λω, the five gates, Fit,
GRAVIS, Position Zero: these are SUM’s terms, carried here as readings of the same facts. Some are derived from the model’s axioms; some are proposed. The biology in this page is offered in the model’s own voice, as interpretation — not as a new result, and not as a request for the laboratory to change its methods.
The honest summary is short. Biology builds and guards the boundary. Molecular recognition is Fit at small scale. Evolution is selection for Fit, channelled into narrow workable ground. The heart, the skin, the genome and felt time each register weight. Violence is measurable, evil is not — and the curves of violence describe the vehicle, while the content requires the recovery of shared ground. And the witness — Position Zero, resting in D∞ — is what all of it is for.
A conclusion: two, or five dimensions?
One last clarification, because the model’s own phrasing invites the question. When SUM says reality has two parts — M₄ and Ϙ — the “two” counts the factors, not the directions. M₄ is already four: three of space and one of time. Ϙ is the fifth, but it is not a fifth direction anyone could point to. It is the qualitative dimension — the arena in which what things are like occurs.
So the count is right both ways at once: two factors, five dimensions. M₅ = M₄ × Ϙ is a product, not a sum — co-presence, not emergence. The measurable world was never without the qualitative one, and the qualitative one never floats free of the measurable. (That the phrase
“the second dimension” arrives independently at more than one reader’s desk is not a coincidence to worry about; it is the model’s own sentence doing its job.)
“Reading science from the second dimension” is a shorthand for reading it
from Ϙ: keeping every measurement exactly as the laboratory made it, and asking alongside it the only question Ϙ adds — what is it like, and what does it weigh? The two investigations meet at the Primaton, the convergence point where scientific and contemplative inquiry address one reality. That meeting is the model’s whole wager, and this page has tried to hold it with discipline: nothing added to the data, nothing subtracted from the second account — and the witness, Position Zero resting in D∞, present at every gate where a living body receives the world.
Toledo, 11 October 2026


Leave a Reply